

This post is mainly claude. My first question related to a paper by Day and Claude Athos which my version of Claude summarized thusly:
The Mathematics of Neutral Evolution and Its Critics: A Technical Summary
Kimura’s neutral theory (1968, 1983) rests on two mathematical pillars that have shaped molecular evolution for half a century.
The Substitution Rate Formula:
In a diploid population of effective size Ne, new neutral mutations arise at rate 2Neμ per generation (where μ is the per-site mutation rate). Each mutation has fixation probability 1/(2Ne) under pure drift. The substitution rate becomes:
k = 2Neμ × 1/(2Ne) = μ
This elegant result—that neutral substitution rates equal mutation rates independent of population size—became the foundation for molecular clock dating and divergence time estimation.
The Diversity Formula:
At mutation-drift equilibrium, expected pairwise nucleotide diversity is:
π = 4Neμ
This relationship provides the standard method for estimating effective population size from genetic data: Ne = π/(4μ).
Haldane’s Cost of Selection
Haldane (1957) addressed a different question: how many beneficial substitutions can occur simultaneously? His “cost of selection” argument calculated that each allele substitution requires a cumulative genetic load (selective deaths) of approximately:
C ≈ 2ln(1/p0)
For a new mutation starting at frequency p0 = 1/(2N), this yields C ≈ 2ln(2N) ≈ 10-30 “substitution-equivalents” for typical population sizes. Since organisms have finite reproductive capacity, Haldane argued this limits substitution rates to roughly 1 per 300 generations—the so-called “speed limit” on adaptive evolution.
Fixation Probability Under Selection
For a beneficial allele with selective advantage s in a population of size Ne, the fixation probability is approximately:
π(s) ≈ 2s/ρ²
where ρ² is the offspring variance (ρ² = 1 for Wright-Fisher populations). The Boenkost et al. (2021) paper proves this formula holds rigorously in the regime of “moderately strong selection” where N^(-1/2+η) ≤ sN ≤ N^(-η) for Cannings models with Dirichlet-type offspring distributions.
The time to fixation for a beneficial allele, conditional on fixation occurring, scales as:
t_fix ≈ (2/s)ln(2N) [for strong selection, s >> 1/(2Ne)]
t_fix ≈ 4Ne [for weak selection, s << 1/(2Ne)]
The Two-Ne Problem
Day & Athos (2025) identify a fundamental contradiction in Kimura’s k = μ derivation. The formula requires Ne to represent two distinct biological processes:
Mutation supply: 2Neμ mutations arise per generation—a biochemical process occurring during DNA replication in census individuals
Fixation probability: 1/(2Ne) represents drift dynamics, determined by variance in reproductive success
These processes operate on different population scales. Mutations originate in all reproducing individuals (census N), but drift is determined by effective size Ne, which incorporates reproductive variance, population structure, and selection. When N >> Ne (as observed empirically), the cancellation fails:
k = 2Nμ × 1/(2Ne) = (N/Ne)μ
This predicts substitution rates should exceed mutation rates by the N/Ne ratio.
Empirical Discrepancies
Day & Athos document systematic census/Ne discrepancies across three mammalian species:
Chimpanzees: Census N ≈ 1,000,000; diversity-derived Ne ≈ 21,700 (ratio 46:1)
Gorillas: Census N ≈ 500,000; diversity-derived Ne ≈ 26,300 (ratio 19:1)
Killer whales: Census N ≈ 50,000+; very low Ne (ratio >10:1)
Using census N to predict diversity via π = 4Nμ over-predicts observed diversity by these same factors. The standard resolution invokes:
π = 4Neμ where Ne = N/(variance inflation factor)
This makes Ne a fitting parameter defined by Ne* = π/(4μ), creating circularity: the “prediction” π = 4Ne*μ reduces to π = π.
The Generation Overlap Correction
Day & Athos (2025a) introduce the Bio-Cycle model incorporating a generation overlap correction factor d:
Δp_t = d · s · p_t(1-p_t)
where d < 1 reflects that not all individuals in generation t compete with generation t+1 in species with overlapping generations. Classical models assume discrete generations (d = 1).
Testing against ancient DNA time series for three loci under positive selection (lactase persistence, SLC45A2, TYR), the Bio-Cycle model with d ≈ 0.45 reduces prediction error by 69% compared to the classical Kimura model. The Kimura model systematically over-predicts final allele frequencies, driving alleles toward near-fixation when observed frequencies remain substantially lower.
The Selective Turnover Coefficient (Day & Athos 2025b) derives d from first principles using reproductive-value-weighted mortality schedules. For Neolithic/Bronze Age demographic conditions (Coale-Demeny life tables), theory predicts d ≈ 0.45-0.53, matching the empirical estimate.
Mathematical Implications
For Fixation Times:
The generation overlap correction implies that effective generation counts in overlapping-generation species are approximately half the nominal counts. For human evolution with 20-year generation times:
Nominal generations over 6 Myr: 300,000
Effective generations (d=0.45): 135,000
This has profound implications for evolutionary rate estimates and the feasibility of adaptive substitutions over deep time.
For Haldane’s Limit:
With d = 0.45, the effective generation count available for substitutions roughly halves:
Maximum substitutions ≈ (d × t_available)/(300 gen/substitution)
For Neanderthal divergence (20,000 nominal generations):
Classical limit: 67 substitutions
Bio-Cycle correction: 30 substitutions
For Mutation-Drift Balance:
The diversity formula becomes:
π = 4Neμ where Ne represents effective drift dynamics
but mutation supply remains tied to census N. The relationship Ne/N captures the combined effects of:
Reproductive variance: Var(offspring) > Poisson expectation
Population structure: subdivision reduces effective size
Linked selection: background selection and hitchhiking
Temporal variance: bottlenecks and fluctuations
Standard theory attributes 20-50× reductions in Ne/N to these “neutral” processes, but Day & Athos argue that invoking such massive reductions requires pervasive selection—undermining the neutrality assumption.
The Degeneracy Problem
The key mathematical issue is that Ne appears in multiple formulas but is operationally defined by back-calculation from diversity:
Ne := π/(4μ)
When this Ne is then used to “predict” diversity, fixation probabilities, or substitution rates, the model has no independent predictive content. Any observed diversity can be accommodated by adjusting Ne post-hoc.
Waples (2025) acknowledges this: “the effective population size is usually estimated empirically with respect to the amount of within-species genetic diversity divided by the mutation rate, yielding a coalescent effective population size that reflects the cumulative effects of genetic drift, background selection, and genetic hitchhiking.”
The problem is not logical unfalsifiability in the strict Popperian sense—one could imagine independent Ne measurements from pedigree variance or temporal methods. Rather, the model is degenerately parameterized: it has more free parameters than data points to constrain them, allowing post-hoc accommodation of any observation.
Conclusion
The mathematical foundations of neutral theory rest on elegant formulas that conceal interpretational ambiguities. The Ne parameter simultaneously represents mutation supply (tied to census N), drift dynamics (Ne << N due to reproductive variance), and a fitting parameter for observed diversity. The Bio-Cycle correction demonstrates that classical discrete-generation assumptions systematically mis-predict allele frequency trajectories in ancient DNA, suggesting that fundamental assumptions about generation structure require revision. Whether these tensions represent fatal flaws or opportunities for theoretical refinement remains an active area of investigation.
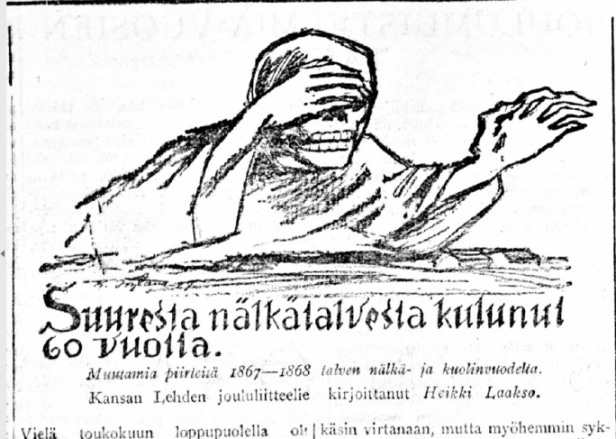
What has happened, historically, to humans, is that the populations collapse. This causes bottlenecks. This is speculated to have occurred in ancient times and famines happened in more marginal lands until very recently. Finland is an example:
Finland has a long history of famines: currently available Finnish population series document famines in 1675–9, in the 1690s (with a population decline of 20.6% in 1696–7), in 1709–10, in the early 1740s, and more regionally delineated crises during the 1830s and 1850s, with continued food security crises related to harvest failure well into the 20th century. What makes the Finnish famine of the 1860s stand out was not only its relatively late occurrence (approximately 120 years after the previous large-scale domestic famine, and some 90 years after the last substantial famine in neighbouring Sweden) but also its magnitude, with a loss of nearly 10% of the pre-famine population. The Finnish famine of the 1860s took place in a poor country: in 1820 Finland had a per capita income level that was only 40% of the UK and 75% of Sweden.
When I got Claude to analyse this, the severity of this did not make that much difference to the genetic makeup of the Finnish population compared with Swedish. This is the summary of the math and the example.
# Population Bottleneck Mathematics: A Technical Summary
## Core Concepts
A population bottleneck occurs when population size drops suddenly from N₀ to N_b (bottleneck size), remains at N_b for t_b generations, then recovers to N₀ or a new equilibrium.
## Effective Population Size Across Bottlenecks
The harmonic mean formula gives long-term effective population size across variable epochs (Crow & Kimura 1970):
**1/N_e = (1/T) Σ(t_i/N_i)**
For a simple bottleneck of duration t_b at size N_b, followed by T - t_b generations at size N₀:
**1/N_e = (t_b/N_b + (T - t_b)/N₀) / T**
Critical insight: Even brief severe bottlenecks dramatically reduce long-term N_e because the harmonic mean is dominated by the smallest value.
## Heterozygosity Loss
Expected heterozygosity after t generations at population size N follows (Kimura 1983):
**H_t = H₀(1 - 1/(2N))^t**
For a single-generation bottleneck:
**ΔH/H₀ = 1/(2N_b)**
Example: A bottleneck to N_b = 1,000 individuals causes ~0.05% heterozygosity loss per generation. For severe bottlenecks (N_b < 100), losses become substantial: N_b = 50 loses ~1% per generation.
## Allele Loss Probability
For a neutral allele at frequency p before the bottleneck, probability of loss during sampling of N_b diploid individuals (Ewens 2004):
**P(loss) = (1-p)^(2N_b)**
For rare alleles (p << 1): **P(loss) ≈ e^(-2N_bp)**
Example: An allele at p = 0.01 has 82% probability of loss if N_b = 10, but only 13% if N_b = 100. Rare alleles (p < 0.001) are extremely vulnerable.
## Multiple Bottlenecks
For k sequential bottlenecks with sizes N_b1, N_b2, ..., N_bk and durations t_b1, t_b2, ..., t_bk:
**1/N_e = (1/T)[Σ(t_bi/N_bi) + (T - Σt_bi)/N₀]**
Cumulative heterozygosity loss is multiplicative:
**H_final = H₀ Π(1 - 1/(2N_bi))^(t_bi)**
## Coalescent Theory Framework
Under the standard coalescent (Kingman 1982), expected time to most recent common ancestor (TMRCA) for two lineages is 2N_e generations. During a bottleneck, probability two lineages coalesce during bottleneck phase:
**P(coalesce in bottleneck) ≈ t_b/(2N_b)**
This creates “star-like” genealogies where many lineages trace to few ancestors during the bottleneck period.
## Time to Recovery
After a bottleneck, heterozygosity recovers toward equilibrium π = 4N₀μ (for diploids) following:
**H_t = H_eq - (H_eq - H_b)e^(-t/(2N₀))**
Recovery timescale: **τ ≈ 4N₀ generations**
For N₀ = 10,000, full recovery requires ~40,000 generations—far longer than most bottleneck durations. This asymmetry (rapid loss, slow recovery) explains persistent signatures of historical bottlenecks.
## Empirical Example: Finnish Famines
Finnish famines (1696-1697: 20% mortality; 1866-1868: 10% mortality) with N₀ ~ 500,000 produced minimal genetic impact. Even three events with t_b = 1 generation each:
**H_final/H₀ = (1 - 1/(2×400,000))³ ≈ 0.9999925**
**Cumulative diversity loss: ~0.0075%**—negligible because N_b remained large.
## Critical Parameters
Genetic impact depends on:
1. **Severity**: N_b/N₀ ratio (lower = worse)
2. **Duration**: t_b (longer = worse)
3. **Frequency**: Number of events
4. **Recovery time**: Intervals between events
**Conclusion**: Substantial genetic effects require N_b << 10,000 and/or t_b >> 10 generations.
## References
Crow JF, Kimura M (1970). *An Introduction to Population Genetics Theory*. Harper & Row.
Ewens WJ (2004). *Mathematical Population Genetics I: Theoretical Introduction* (2nd ed.). Springer.
Kimura M (1983). *The Neutral Theory of Molecular Evolution*. Cambridge University Press.
Kingman JFC (1982). On the genealogy of large populations. *Journal of Applied Probability* 19:27-43.
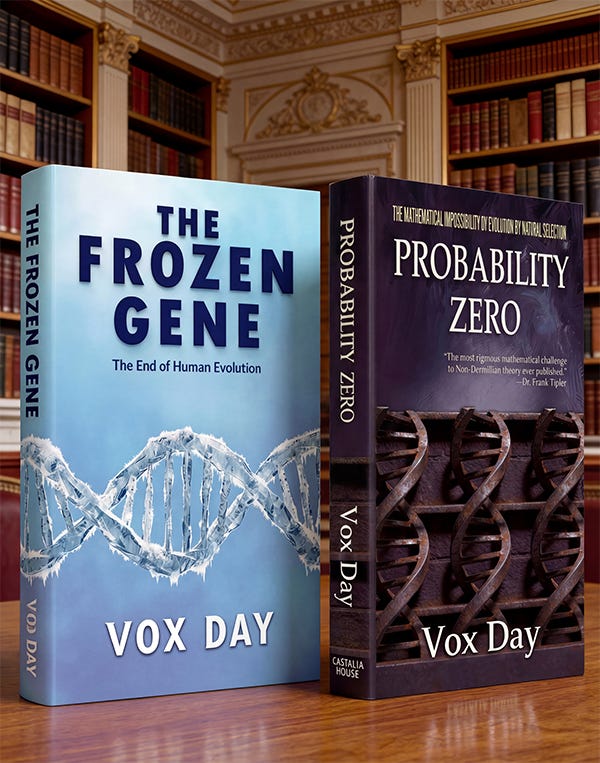
This is heading to where Mr Day is going. He does the math. Repeatedly, and across species. Matthew Littlefield had reviewed the book again, reminding us that his previous book “The Irrational Atheist” also did the math to disprove numbers used as rhetoric.
You hear much less today about how much war is caused by religion, have you noticed that? You are more like to hear people say that all wars are bankers wars, or the result of imperialism or something like that. This is in part because of Day’s 2008 book. It changed the cultural understanding of what the fundamental causes of war are, and took away one of the so-called New Atheists favourite weapons. The reason he was able to do this was simple: he did the math. He did what none of us thought to do, he sat down and actually calculated, to the best of our history knowledge at the time, how many wars were known to be caused by religion. And this simple examination pulled apart the threads of a powerful rhetorical argument against Christianity. Vox has done this again with Probability Zero: The Mathematical Impossibility of Evolution by Natural Selection. The premise of Vox Day’s argument is relatively simple: if something happens in the physical world then it can be quantified. This is a simple enough concept. The way it applies to Day’s book is as such: if evolution is happening, what is the average rate of evolution? This is the thread which Day has pulled on to bring down the whole Evolution by Natural Selection edifice. A simple question to an evolutionary biologist in a debate in 2019, that could not be answered, has turned into a demonstration of the impossibility of evolution via any proposed natural means. The mechanisms simply do not work. They do not have the horse power to achieve what we were told they could achieve.
I have not read his second book fully yet, but in the next post I’m going to go through the issues relating to what happens when a population has a massive die-off, and how it does not explain what is happening.